2.wle
wle 时间:2021-02-28 阅读:()
AmplicationeciencyofthermostableDNApolymerasesBahramArezi,WeimeiXing,JosephA.
Sorge,andHollyH.
Hogrefe*StratageneCloningSystems,11011NorthTorreyPinesRoad,LaJolla,CA92037,USAReceived6May2003AbstractTheamplicationecienciesofseveralpolymerasechainreaction(PCR)enzymeswerecomparedusingreal-timequantitativePCRwithSYBRGreenIdetection.
AmplicationdatacollectedduringtheexponentialphaseofPCRarehighlyreproducible,andPCRenzymeperformancecomparisonsbaseduponeciencymeasurementsareconsiderablymoreaccuratethanthosebasedonendpointanalysis.
DNApolymeraseecienciesweredeterminedunderidenticalconditionsusingvedierentamplicontemplatesthatvariedinlengthorpercentageGCcontent.
Pfu-andTaq-basedformulationsshowedsimilareciencieswhenamplifyingshortertargets(PfuUltraPPfu/Taqblends(Herculase,HerculaseHotstart)>Taq-onlyformations(PlatinumTaq,Sure-StartTaq)(leastresistant).
AlthoughsomeDNApolymerases(e.
g.
,Pfu)wereinsensitivetohighercon-centrationsofSYBRGreenI,weusedeither1:60,000or1:120,000dilutionsofSYBRGreenI(nalinPCR:4.
2-or8.
3107(v/v))inQ-PCRs.
TheseSYBRGreenIconcentrationsgeneratedsucientsignalintensityfordetectionandanalysisandresultedinsimilarampli-cationeciencieswhenamplifyingthesametarget(datanotshown).
AmplicationeciencycomparisonsfordierenttargetlengthsEciencywasquantiedinamplicationreactionsemployingPCRampliconsastemplate.
Usingawiderangeofamplicontemplateamounts(102–107copies)allowedustoobtainastronglinearcorrelationbe-tweenCTsandinitialcopynumber(ahighregressioncoecient)andthereforeahighdegreeofreproduc-ibility.
Toexaminetheeectoftargetlengthontheampli-cationeciencyofDNApolymerases,primerAT-FwasusedincombinationwithprimersAT-R1,AT-R2,andAT-R3toamplify0.
9-,2.
6-,and3.
9-kbfragments,respectively.
PCRamplicationswereperformedwithnestedprimersusingeachDNApolymeraseinitsopti-malPCRbuer.
AllPCRparameterswereidentical,exceptthatPCRenzymeamount,Mg2concentration,andPCRcyclingparameterswereadjustedaccordingtothemanufacturersrecommendations(seeMaterialsandmethods).
Fig.
2showsanexampleofanamplicationplotandstandardcurveforHerculaseHotstartDNApolymerase.
AmplicationeciencieswerecalculatedfromtheslopeofstandardcurvesasE101=slope1.
Table3summarizestheamplicationecienciesofvariousPCRenzymesasafunctionofampliconsize.
ThetwohotstartversionsofTaqexhibitedsimilaramplicationeciencies(82–83%,0.
9kb;62–66%,2.
6kb),eventhoughreversibleinactivationwasachievedbyverydierentmeans(chemicalmodication,Sure-StartTaq;antibodyneutralization,PlatinumTaq).
De-spitetheuseoflongerextensiontimes(1min/kb),amplicationeciencydecreasedwithincreasingam-pliconsizeabove1–2kb.
Infact,amplicationeciencycouldnotbeaccuratelydeterminedforthe3.
9-kbtargetasbothTaqformulationsproducedsmearsandmultiplebands.
LikeTaq,theamplicationeciencyofPfuDNApolymerasedecreasedwithincreasingtemplatesizeabove1–2kb(78%,0.
9kb;71%,2.
6kb;49%,3.
9kb).
Incontrast,theamplicationecienciesofPfuformula-tionswithdUTPase(PfuTurbo,PfuUltra,Herculase)weresignicantlyhigherforPCRsemployingthe2.
6-kbFig.
1.
InhibitoryeectsofhighSYBRGreenIconcentrationsonDNApolymerases.
PfuTurboHotstartDNApolymerasewasusedtoamplifythe0.
9-kbtarget,asdescribedunderMaterialsandmethods.
ReactionsateachSYBRdilutionwereperformedinduplicate.
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235229(80–84%vs71%forPfuand62–66%forTaq)and3.
9-kb(66–74%vs49%forPfu)amplicons.
PfuUltra,whichisformulatedwithPfumutantandpossesseshigherproofreadingactivity[20],demonstratessomewhatloweramplicationeciencies(2.
3to8%lower)thanPfuTurbo.
NeutralizingmonoclonalantibodieshadminimaleectsontheamplicationeciencyofhotstartPfuformulations(variedwithin0.
9–4.
8%).
Table2SYBRGreenIsensitivityofDNApolymerasesPolymeraseAmpliconsize(GCcontent)Dilutions(1/1000)1:101:201:401:601:1201:240Pfu545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuTurbo545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuTurbo545bp(78%Hotstart545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuUltra545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PlatinumPfx545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%)N/AN/AN/AN/AN/AN/ATgo545bp(78%)N/AN/AN/AN/AN/AN/A545bp(45%0.
9kb(56%)N/AN/AN/AN/AN/AN/ASureStartTaq545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)N/AN/AN/AN/AN/AN/APlatinumTaq545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)N/AN/AN/AN/AN/AN/AHerculase545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%Herculase545bp(78%Hotstart545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)),Inhibitionshownas>2CTdelayandweakerornobandonthegel;)/+,slightinhibitionshownas>0.
5CTand62CTdelay;++,noinhibition(optimalamplication);N/A,nodataavailable(nospecicproductorthepresenceofsmearormultiplebands).
230B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235WealsoexaminedotherarchaealDNApolymerasessuchasKOD(PlatinumPfx)andTgoDNApolyme-rases.
PlatinumPfxDNApolymeraseampliedthe0.
9-kbfragmentwith66%amplicationeciency,whichissignicantlylowerthantheeciencyofPfualone(78%)orwithdUTPase(83%).
EcienciescouldnotbeFig.
2.
Real-timePCRamplicationof10-foldserialdilutionsofthe545-bpamplicon.
HerculaseHotstartDNApolymerasewasusedtoamplifythe545-bpampliconwith45%CGcontent,asdescribedunderMaterialsandmethods.
(A)Real-timePCRamplicationplot;(B)PCRproductsampliedfrom5107to5102(10-foldserialdilutions,lanes1–6)molecules/llbygelelectrophoresis;(C)standardcurvewith(R2)valueandregressiontequationindicated.
EachPCRwasperformedinquadruplicate.
NTC,no-templatecontrol.
Table3Amplicationeciencies(%)asafunctionoftargetlengthPolymeraseTargetlength(kb)0.
92.
63.
9Pfu78.
81.
771.
21.
649.
11.
7PfuTurbo83.
20.
683.
71.
174.
40.
6PfuTurboHotstart82.
11.
981.
61.
070.
81.
0PfuUltra80.
91.
3180.
41.
5666.
41.
21PlatinumPfx66.
11.
6N/AN/ATgoN/AN/AN/ASureStartTaq82.
61.
262.
31.
2N/APlatinumTaq81.
90.
465.
72.
0N/AHerculase89.
71.
281.
72.
071.
61.
8HerculaseHotstart90.
71.
080.
81.
873.
50.
3Amplicationecienciesaretheaveragesobtainedfromatleastthreeindependentexperimentswiththestandarddeviationsindicated.
Betweenfourandsixserialtemplatedilutionswereusedineachexperiment(eachdilutionwaspreparedintriplicateorquadruplicate).
N/A,nodataavailable(nospecicPCRproductorgenerationofsmearormultipleproducts).
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235231determinedforlongertargetsusingPlatinumPfx(>0.
9-kbfragments)orTgo(>0.
6-kbfragments)DNApoly-meraseduetofailuretoamplify.
ComparedtoPfuTurbo,HerculasecontainsaminorpercentageofTaqandauniquePCRbuer,whichhavebeenshownpreviouslytoenhancethetarget-lengthca-pabilityofPfuinthepresenceofdUTPase(increasesfrom19to37kbforgenomictargets)[20].
Withoneexception(the0.
9-kbsystem),HerculaseandPfuTurboDNApolymerasesexhibitedsimilaramplicatione-cienciesovertherangeoftargetssizesexamined.
Pre-sumably,dierencesinamplicationeciencywouldbeapparentincomparisonsemployinglongeramplicons.
VariationofamplicationeciencywithpercentageGCcontentToaddressthecontributionofGCcontentonam-plicationeciency,weemployedtwo545-bpampli-conswithidenticalPCRprimerannealingsequences,buteither45or78%GCcontent(seeMaterialsandmethods).
ToenhanceamplicationoftheGC-richtarget,DMSOwasadded(1to15%(v/v);1%incre-ments),andtheoptimalconcentrationthatgeneratedthelowestCTswasdeterminedforeachDNApoly-meraseexamined.
Theresultswereasfollows:Pfu(6–10%),PfuTurbo(Hotstart)(7–11%),PfuUltra(6–9%),SureStartTaq(8–10%),PlatinumTaq(7–8%),andHer-culase(Hotstart)(6–10%).
Asanexample,theDMSOtitrationforPfuTurboisshowninFig.
3.
AllDNApolymerasesampliedthe78%GCtargetoptimallyat8%DMSO,althougheachexhibitedauniqueDMSOsensitivityprole.
WiththeexceptionofPlatinumPfx,amplicationeciencywasdeterminedfromPCRsemployingeither8%DMSO(78%GCamplicon)or0%DMSO(45%GCamplicon).
DMSOdidnotaecteciencymeasurementsforthe45%GCtarget(datanotshown).
Inourhands,PlatinumPfxgeneratedweakandmultiplePCRproductsevenwhenDMSOwasadded.
Therefore,theproprietaryPCRxsolutionrec-ommendedbythemanufacturerwasusedinsteadtosuccessfullyamplifytheGC-richamplicon(2.
5nalconcentration).
AsshowninTable4,allDNApolymerasesampliedthe78%GCampliconwithsignicantlylowereciencycomparedtothe45%GCamplicon.
Pfuexhibitedaneciencyof77.
2%whenamplifyingthe45%GCtarget.
However,whenGCcontentincreasedto78%,theam-plicationeciencydroppedto51.
3%.
Likewise,Sure-StartTaq,PlatinumTaq,PfuTurbo,andHerculaseexhibitedsimilareciencieswhenamplifyingthe45%GCtarget(75to80%).
However,withtheGC-richamplicon,amplicationeciencywassignicantlylowerandvariedasfollows:(highesteciency):54–55%;PfuTurbo(Hotstart),Herculase(Hotstart)>51%;Pfu>42–44%;PfuUltra,SureStartTaq,PlatinumTaq>29%;Pfx(lowesteciency).
EveninthepresenceofDMSO(upto15%(v/v)),TgoDNApolymerasegeneratedsmearswhileamplifyingthe78%GCtarget,andthusamplicationeciencycouldnotbedetermined(datanotshown).
DiscussionUnlikemostenzymaticreactions,PCRisanexpo-nentialprocessandthereforeverysmallchangesinamplicationeciency,E,canresultindramaticdierencesintheamountofnalproduct,eveniftheinitialnumberoftargetmoleculesisthesame.
Forexample,ifE74:7%(e.
g.
,PfuTurbo,3.
9-kbFig.
3.
Real-timePCRamplicationinthepresenceofvaryingDMSOamounts.
PfuTurboDNApolymerasewasusedtoamplifythe545-bpampliconwith78%CGcontentinthepresenceofdierentamountsofDMSO(0–15%(v/v),in1%increments)(seeMaterialsandmethods).
Table4Amplicationeciencies(%)asafunctionofGCcontentPolymeraseGCcontent45%78%aPfu77.
21.
851.
31.
6PfuTurbo79.
91.
655.
21.
8PfuTurboHotstart75.
11.
154.
51.
9PfuUltra70.
81.
944.
11.
8PlatinumPfx61.
21.
128.
70.
7bTgo56.
91.
9N/ASureStartTaq78.
71.
542.
10.
4PlatinumTaq78.
50.
543.
30.
5Herculase79.
71.
154.
71.
3HerculaseHotstart80.
41.
254.
50.
8Amplicationecienciesaretheaveragesobtainedfromatleastthreeindependentexperimentswiththestandarddeviationsindicated.
Betweenfourandsixserialtemplatedilutionswereusedineachexperiment(eachdilutionwaspreparedintriplicateorquadruplicate).
N/A,nodataavailable(generationofsmearormultipleproducts).
a8%DMSOwasusedintheamplicationofthistarget.
bPCRxsolutionwasaddedaccordingtothemanufacturersrecommendation.
232B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235fragment)andn30,thenNN010:74730or1.
86107N0.
Inotherwords,after30cycles,thisPCRwouldtheoreticallyproducea1.
86107-foldincreaseintheamountoftargetmolecules.
However,ifE49:1%(e.
g.
,Pfu,3.
9-kbfragment),after30cycles,thetargetwouldbeampliedonly1.
6105timesbyPCR.
Thusa25.
6%dierenceinamplicatione-ciencyleadstoa116-folddierenceintheamountofnalproduct.
PCRproductyieldisgenerallythemostimportantparameterconsideredwhenselectingaPCRenzymeforamplication.
Despiteitsimportance,verylittlecom-parativeinformationexistswithregardtoamplicationecienciesofcommercialPCRenzymes.
Inthisstudy,wedeterminedtheamplicationeciencyof10dierentDNApolymeraseformulationsunderoptimalcondi-tions(enzymeamount,PCRbuer,extensiontempera-ture)usingidenticalreactionparameters(primerandtemplateconcentrations,cyclingregimen).
SignicantdierencesinthePCRenzymeeciencywereapparentincarefullycontrolledcomparisonsemployingvetemplatesofvaryinglengthandGCcontent.
AllDNApolymerasesexaminedexhibitedroughlysimilareciencieswhenamplifyingsmallerfragments(1–2kb)orGC-richamplicons.
Forexample,Table5showsthenumberofcyclesrequiredtoachieve106-foldamplicationusingtheeciencyvaluesdeter-B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235233minedforthe545-(Table4)and2.
6-kb(Table3)am-plicons.
AlthoughallDNApolymerasescanamplifythelow%-GCamplicons106-foldwithin30cycles,thede-siredlevelofamplicationisachieved1to7cyclesearlier,dependingontheDNApolymeraseemployed.
Forexample,the2.
6-kbampliconcanbeamplied106-foldin23cyclesusingPfuTurbo,PfuUltra,andHercu-laseDNApolymerases,comparedto29cyclesusingSureStartTaqDNApolymerase.
However,dependingonthetargetDNAsequence,theminimumnumberofcyclesrequiredtoachieve106-foldamplicationmaygreatlyexceed30cycles.
Forexample,dependingontheDNApolymeraseemployed,anadditional7to26cyclesisrequiredtoamplifythe78%GCampliconcomparedtothe45%GCamplicon(Table5).
ThehigherthenumberofPCRcycles,thehigherthechancesofam-plifyingundesiredproducts,suchasprimerdimers.
Inadditiontoeciency,PCRenzymedelityisanotherimportantconsiderationwhenamplifyinglongtargets(>1kb),sincethepercentageofclonescontainingerrorsincreasesproportionallywithincreasingampliconsize.
AsshowninTable5,Pfu+dUTPaseformulations(PfuUltra,PfuTurbo)areexpectedtoamplifylongertargetswithboththefewestnumberofcyclesandthefewestpolymerase-inducederrors.
AnumberofmodicationstothebasicPCRformatincludingadditivessuchasformamide[23],DMSO[24,25],betaine[26],etc.
havebeenpublishedinanat-tempttoincreaseamplicationeciencyandspecicity,regardlessofampliconlengthorcomposition.
Real-timePCRmethods,suchasthosedescribedinthisreport,representapowerfultoolformonitoringeortstoop-timizeamplicationeciency.
ThedatageneratedbythisprotocolarecollectedattheexponentialphaseofPCRandthereforedemonstratehighreproducibilitycomparedtoendpointanalysisbygelelectrophoresis.
QuantitativemethodsshowpromiseinthedevelopmentandqualitycontrolofPCRenzyme/buerformulationstoensureconsistencyandmaximalperformance.
AcknowledgmentsTheauthorsthankDrs.
VanessaGurtu,MadhushreeGhosh,andReinholdMuellerforcriticalreadingofthismanuscript.
References[1]K.
Mullis,F.
Faloona,S.
Scharf,R.
Saiki,G.
Horn,H.
Erlich,SpecicenzymaticamplicationofDNAinvitro:thepolymerasechainreaction,ColdSpringHarb.
Symp.
Quant.
Biol.
51(1)(1986)263–273.
[2]S.
A.
Bustin,AbsolutequanticationofmRNAusingreal-timereversetranscriptionpolymerasechainreactionassays,J.
Mol.
Endocrinol.
25(2000)169–193.
[3]R.
S.
Cha,W.
G.
Thilly,Specicity,eciency,anddelityofPCR,in:C.
W.
Dieenbach,G.
S.
Dveksler(Eds.
),PCRPrimer:ALaboratoryManual,ColdSpringHarborLaboratoryPress,ColdSpringHarbor,NY,1995.
[4]R.
J.
Wiesner,DirectquanticationofpicomolarconcentrationsofmRNAsbymathematicalanalysisofareversetranscription/exponentialpolymerasechainreactionassay,NucleicAcidsRes.
20(1992)5863–5864.
[5]R.
Higuchi,C.
Fockler,G.
Dollinger,R.
Watson,KineticPCRanalysis:real-timemonitoringofDNAamplicationreactions,Biotechnology11(1993)1026–1030.
[6]L.
L.
Ling,P.
Keohavong,C.
Dias,W.
G.
Thilly,Optimizationofthepolymerasechainreactionwithregardtodelity:modiedT7,Taq,andventDNApolymerases,PCRMethodsAppl.
1(1991)63–69.
[7]A.
M.
Dunning,P.
Talmud,S.
E.
Humphries,Errorsinthepolymerasechainreaction,NucleicAcidsRes.
16(1988)10393.
[8]P.
Keohavong,W.
G.
Thilly,FidelityofDNApolymerasesinDNAamplication,Proc.
Natl.
Acad.
Sci.
USA86(1989)9253–9257.
[9]A.
Karsai,S.
Muller,S.
Platz,M.
T.
Hauser,EvaluationofahomemadeSYBRgreenIreactionmixtureforreal-timePCRTable5VariationofcyclenumberandmutationfrequencywithDNApolymeraseDNApolymeraseErrorrate(mutationperbpperduplication)a545-bpamplicon2.
6-kbampliconPCR-inducedmutantfraction(%)bNumberofcyclesrequiredcPCR-inducedmutantfraction(%)bNumberofcyclesrequiredc45%GC78%GC+additivesPfu1.
310612433726PfuTurbo1.
310612431723PfuUltra4.
31070.
52638223Pfx3.
51064295518NAHerculase2.
8106324321523SureStartTaq8.
0106924394229aFromHogrefeandBorns[20].
bFractionoferror-containingproductsfollowing106-foldamplicationoftheindicatedtargetsequencegiventheDNApolymeraseerrorrate.
MutationfrequencieswerecalculatedusingtheequationmfERbpd,wheremfisthemutationfrequency,ERistheerrorrate,bpisthelengthofthetarget,anddisthenumberoftemplatedoublings[13].
cNumberofcyclesrequiredtoobtain106-foldamplicationgiventheeciencypercycleinTables3and5.
234B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235quanticationofgeneexpression,Biotechniques32(2002)790–792,794–796.
[10]K.
S.
Lundberg,D.
D.
Shoemaker,M.
W.
Adams,J.
M.
Short,J.
A.
Sorge,E.
J.
Mathur,High-delityamplicationusingathermo-stableDNApolymeraseisolatedfromPyrococcusfuriosus,Gene108(1991)1–6.
[11]J.
M.
Flaman,T.
Frebourg,V.
Moreau,F.
Charbonnier,C.
Martin,C.
Ishioka,S.
H.
Friend,R.
Iggo,ArapidPCRdelityassay,NucleicAcidsRes.
22(1994)3259–3260.
[12]W.
M.
Barnes,PCRamplicationofupto35-kbDNAwithhighdelityandhighyieldfromlambdabacteriophagetemplates,Proc.
Natl.
Acad.
Sci.
USA91(1994)2216–2220.
[13]J.
Cline,J.
C.
Braman,H.
H.
Hogrefe,PCRdelityofpfuDNApolymeraseandotherthermostableDNApolymerases,NucleicAcidsRes.
24(1996)3546–3551.
[14]D.
E.
Kellogg,I.
Rybalkin,S.
Chen,N.
Mukhamedova,T.
Vlasik,P.
D.
Siebert,A.
Chenchik,TaqStartAntibody:''hotstart''PCRfacilitatedbyaneutralizingmonoclonalantibodydirectedagainstTaqDNApolymerase,Biotechniques16(1994)1134–1137.
[15]H.
Mizuguchi,M.
Nakatsuji,S.
Fujiwara,M.
Takagi,T.
Imanaka,CharacterizationandapplicationtohotstartPCRofneutralizingmonoclonalantibodiesagainstKODDNApolymer-ase,J.
Biochem.
(Tokyo)126(1999)762–768.
[16]T.
Moretti,B.
Koons,B.
Budowle,EnhancementofPCRamplicationyieldandspecicityusingAmpliTaqGoldDNApolymerase,Biotechniques25(1998)716–722.
[17]M.
A.
Greagg,M.
J.
Fogg,G.
Panayotou,S.
J.
Evans,B.
A.
Connolly,L.
H.
Pearl,Aread-aheadfunctioninarchaealDNApolymerasesdetectspromutagenictemplate-stranduracil,Proc.
Natl.
Acad.
Sci.
USA96(1999)9045–9050.
[18]H.
H.
Hogrefe,C.
J.
Hansen,B.
R.
Scott,K.
B.
Nielson,ArchaealdUTPaseenhancesPCRamplicationswitharchaealDNApolymerasesbypreventingdUTPincorporation,Proc.
Natl.
Acad.
Sci.
USA99(2002)596–601.
[19]M.
Takagi,M.
Nishioka,H.
Kakihara,M.
Kitabayashi,H.
Inoue,B.
Kawakami,M.
Oka,T.
Imanaka,CharacterizationofDNApolymerasefromPyrococcussp.
strainKOD1anditsapplicationtoPCR,Appl.
Environ.
Microbiol.
63(1997)4504–4510.
[20]H.
H.
Hogrefe,M.
Borns,HighdelityPCRenzymes,in:C.
W.
Dieenbach,G.
S.
Dveksler(Eds.
),PCRPrimer:ALaboratoryManual,ColdSpringHarborLaboratoryPress,ColdSpringHarbor,NY,2003.
[21]H.
H.
Hogrefe,J.
Cline,A.
E.
Lovejoy,K.
B.
Nielson,DNApolymerasesfromhyperthermophiles,MethodsEnzymol.
334(2001)91–116.
[22]W.
A.
Al-Soud,P.
Radstrom,PuricationandcharacterizationofPCR-inhibitorycomponentsinbloodcells,J.
Clin.
Microbiol.
39(2001)485–493.
[23]G.
Sarkar,S.
Kapelner,S.
S.
Sommer,Formamidecandramat-icallyimprovethespecicityofPCR,NucleicAcidsRes.
18(1990)7465.
[24]P.
R.
Winship,AnimprovedmethodfordirectlysequencingPCRampliedmaterialusingdimethylsulphoxide,NucleicAcidsRes.
17(1989)1266.
[25]R.
Chakrabarti,C.
E.
Schutt,NovelsulfoxidesfacilitateGC-richtemplateamplication,Biotechniques32(2002)866,868,870–872,874.
[26]W.
Henke,K.
Herdel,K.
Jung,D.
Schnorr,S.
A.
Loening,BetaineimprovesthePCRamplicationofGC-richDNAsequences,NucleicAcidsRes.
25(1997)3957–3958.
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235235
Sorge,andHollyH.
Hogrefe*StratageneCloningSystems,11011NorthTorreyPinesRoad,LaJolla,CA92037,USAReceived6May2003AbstractTheamplicationecienciesofseveralpolymerasechainreaction(PCR)enzymeswerecomparedusingreal-timequantitativePCRwithSYBRGreenIdetection.
AmplicationdatacollectedduringtheexponentialphaseofPCRarehighlyreproducible,andPCRenzymeperformancecomparisonsbaseduponeciencymeasurementsareconsiderablymoreaccuratethanthosebasedonendpointanalysis.
DNApolymeraseecienciesweredeterminedunderidenticalconditionsusingvedierentamplicontemplatesthatvariedinlengthorpercentageGCcontent.
Pfu-andTaq-basedformulationsshowedsimilareciencieswhenamplifyingshortertargets(PfuUltraPPfu/Taqblends(Herculase,HerculaseHotstart)>Taq-onlyformations(PlatinumTaq,Sure-StartTaq)(leastresistant).
AlthoughsomeDNApolymerases(e.
g.
,Pfu)wereinsensitivetohighercon-centrationsofSYBRGreenI,weusedeither1:60,000or1:120,000dilutionsofSYBRGreenI(nalinPCR:4.
2-or8.
3107(v/v))inQ-PCRs.
TheseSYBRGreenIconcentrationsgeneratedsucientsignalintensityfordetectionandanalysisandresultedinsimilarampli-cationeciencieswhenamplifyingthesametarget(datanotshown).
AmplicationeciencycomparisonsfordierenttargetlengthsEciencywasquantiedinamplicationreactionsemployingPCRampliconsastemplate.
Usingawiderangeofamplicontemplateamounts(102–107copies)allowedustoobtainastronglinearcorrelationbe-tweenCTsandinitialcopynumber(ahighregressioncoecient)andthereforeahighdegreeofreproduc-ibility.
Toexaminetheeectoftargetlengthontheampli-cationeciencyofDNApolymerases,primerAT-FwasusedincombinationwithprimersAT-R1,AT-R2,andAT-R3toamplify0.
9-,2.
6-,and3.
9-kbfragments,respectively.
PCRamplicationswereperformedwithnestedprimersusingeachDNApolymeraseinitsopti-malPCRbuer.
AllPCRparameterswereidentical,exceptthatPCRenzymeamount,Mg2concentration,andPCRcyclingparameterswereadjustedaccordingtothemanufacturersrecommendations(seeMaterialsandmethods).
Fig.
2showsanexampleofanamplicationplotandstandardcurveforHerculaseHotstartDNApolymerase.
AmplicationeciencieswerecalculatedfromtheslopeofstandardcurvesasE101=slope1.
Table3summarizestheamplicationecienciesofvariousPCRenzymesasafunctionofampliconsize.
ThetwohotstartversionsofTaqexhibitedsimilaramplicationeciencies(82–83%,0.
9kb;62–66%,2.
6kb),eventhoughreversibleinactivationwasachievedbyverydierentmeans(chemicalmodication,Sure-StartTaq;antibodyneutralization,PlatinumTaq).
De-spitetheuseoflongerextensiontimes(1min/kb),amplicationeciencydecreasedwithincreasingam-pliconsizeabove1–2kb.
Infact,amplicationeciencycouldnotbeaccuratelydeterminedforthe3.
9-kbtargetasbothTaqformulationsproducedsmearsandmultiplebands.
LikeTaq,theamplicationeciencyofPfuDNApolymerasedecreasedwithincreasingtemplatesizeabove1–2kb(78%,0.
9kb;71%,2.
6kb;49%,3.
9kb).
Incontrast,theamplicationecienciesofPfuformula-tionswithdUTPase(PfuTurbo,PfuUltra,Herculase)weresignicantlyhigherforPCRsemployingthe2.
6-kbFig.
1.
InhibitoryeectsofhighSYBRGreenIconcentrationsonDNApolymerases.
PfuTurboHotstartDNApolymerasewasusedtoamplifythe0.
9-kbtarget,asdescribedunderMaterialsandmethods.
ReactionsateachSYBRdilutionwereperformedinduplicate.
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235229(80–84%vs71%forPfuand62–66%forTaq)and3.
9-kb(66–74%vs49%forPfu)amplicons.
PfuUltra,whichisformulatedwithPfumutantandpossesseshigherproofreadingactivity[20],demonstratessomewhatloweramplicationeciencies(2.
3to8%lower)thanPfuTurbo.
NeutralizingmonoclonalantibodieshadminimaleectsontheamplicationeciencyofhotstartPfuformulations(variedwithin0.
9–4.
8%).
Table2SYBRGreenIsensitivityofDNApolymerasesPolymeraseAmpliconsize(GCcontent)Dilutions(1/1000)1:101:201:401:601:1201:240Pfu545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuTurbo545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuTurbo545bp(78%Hotstart545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PfuUltra545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%PlatinumPfx545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%)N/AN/AN/AN/AN/AN/ATgo545bp(78%)N/AN/AN/AN/AN/AN/A545bp(45%0.
9kb(56%)N/AN/AN/AN/AN/AN/ASureStartTaq545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)N/AN/AN/AN/AN/AN/APlatinumTaq545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)N/AN/AN/AN/AN/AN/AHerculase545bp(78%545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%Herculase545bp(78%Hotstart545bp(45%0.
9kb(56%2.
6kb(56%3.
9kb(53%)),Inhibitionshownas>2CTdelayandweakerornobandonthegel;)/+,slightinhibitionshownas>0.
5CTand62CTdelay;++,noinhibition(optimalamplication);N/A,nodataavailable(nospecicproductorthepresenceofsmearormultiplebands).
230B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235WealsoexaminedotherarchaealDNApolymerasessuchasKOD(PlatinumPfx)andTgoDNApolyme-rases.
PlatinumPfxDNApolymeraseampliedthe0.
9-kbfragmentwith66%amplicationeciency,whichissignicantlylowerthantheeciencyofPfualone(78%)orwithdUTPase(83%).
EcienciescouldnotbeFig.
2.
Real-timePCRamplicationof10-foldserialdilutionsofthe545-bpamplicon.
HerculaseHotstartDNApolymerasewasusedtoamplifythe545-bpampliconwith45%CGcontent,asdescribedunderMaterialsandmethods.
(A)Real-timePCRamplicationplot;(B)PCRproductsampliedfrom5107to5102(10-foldserialdilutions,lanes1–6)molecules/llbygelelectrophoresis;(C)standardcurvewith(R2)valueandregressiontequationindicated.
EachPCRwasperformedinquadruplicate.
NTC,no-templatecontrol.
Table3Amplicationeciencies(%)asafunctionoftargetlengthPolymeraseTargetlength(kb)0.
92.
63.
9Pfu78.
81.
771.
21.
649.
11.
7PfuTurbo83.
20.
683.
71.
174.
40.
6PfuTurboHotstart82.
11.
981.
61.
070.
81.
0PfuUltra80.
91.
3180.
41.
5666.
41.
21PlatinumPfx66.
11.
6N/AN/ATgoN/AN/AN/ASureStartTaq82.
61.
262.
31.
2N/APlatinumTaq81.
90.
465.
72.
0N/AHerculase89.
71.
281.
72.
071.
61.
8HerculaseHotstart90.
71.
080.
81.
873.
50.
3Amplicationecienciesaretheaveragesobtainedfromatleastthreeindependentexperimentswiththestandarddeviationsindicated.
Betweenfourandsixserialtemplatedilutionswereusedineachexperiment(eachdilutionwaspreparedintriplicateorquadruplicate).
N/A,nodataavailable(nospecicPCRproductorgenerationofsmearormultipleproducts).
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235231determinedforlongertargetsusingPlatinumPfx(>0.
9-kbfragments)orTgo(>0.
6-kbfragments)DNApoly-meraseduetofailuretoamplify.
ComparedtoPfuTurbo,HerculasecontainsaminorpercentageofTaqandauniquePCRbuer,whichhavebeenshownpreviouslytoenhancethetarget-lengthca-pabilityofPfuinthepresenceofdUTPase(increasesfrom19to37kbforgenomictargets)[20].
Withoneexception(the0.
9-kbsystem),HerculaseandPfuTurboDNApolymerasesexhibitedsimilaramplicatione-cienciesovertherangeoftargetssizesexamined.
Pre-sumably,dierencesinamplicationeciencywouldbeapparentincomparisonsemployinglongeramplicons.
VariationofamplicationeciencywithpercentageGCcontentToaddressthecontributionofGCcontentonam-plicationeciency,weemployedtwo545-bpampli-conswithidenticalPCRprimerannealingsequences,buteither45or78%GCcontent(seeMaterialsandmethods).
ToenhanceamplicationoftheGC-richtarget,DMSOwasadded(1to15%(v/v);1%incre-ments),andtheoptimalconcentrationthatgeneratedthelowestCTswasdeterminedforeachDNApoly-meraseexamined.
Theresultswereasfollows:Pfu(6–10%),PfuTurbo(Hotstart)(7–11%),PfuUltra(6–9%),SureStartTaq(8–10%),PlatinumTaq(7–8%),andHer-culase(Hotstart)(6–10%).
Asanexample,theDMSOtitrationforPfuTurboisshowninFig.
3.
AllDNApolymerasesampliedthe78%GCtargetoptimallyat8%DMSO,althougheachexhibitedauniqueDMSOsensitivityprole.
WiththeexceptionofPlatinumPfx,amplicationeciencywasdeterminedfromPCRsemployingeither8%DMSO(78%GCamplicon)or0%DMSO(45%GCamplicon).
DMSOdidnotaecteciencymeasurementsforthe45%GCtarget(datanotshown).
Inourhands,PlatinumPfxgeneratedweakandmultiplePCRproductsevenwhenDMSOwasadded.
Therefore,theproprietaryPCRxsolutionrec-ommendedbythemanufacturerwasusedinsteadtosuccessfullyamplifytheGC-richamplicon(2.
5nalconcentration).
AsshowninTable4,allDNApolymerasesampliedthe78%GCampliconwithsignicantlylowereciencycomparedtothe45%GCamplicon.
Pfuexhibitedaneciencyof77.
2%whenamplifyingthe45%GCtarget.
However,whenGCcontentincreasedto78%,theam-plicationeciencydroppedto51.
3%.
Likewise,Sure-StartTaq,PlatinumTaq,PfuTurbo,andHerculaseexhibitedsimilareciencieswhenamplifyingthe45%GCtarget(75to80%).
However,withtheGC-richamplicon,amplicationeciencywassignicantlylowerandvariedasfollows:(highesteciency):54–55%;PfuTurbo(Hotstart),Herculase(Hotstart)>51%;Pfu>42–44%;PfuUltra,SureStartTaq,PlatinumTaq>29%;Pfx(lowesteciency).
EveninthepresenceofDMSO(upto15%(v/v)),TgoDNApolymerasegeneratedsmearswhileamplifyingthe78%GCtarget,andthusamplicationeciencycouldnotbedetermined(datanotshown).
DiscussionUnlikemostenzymaticreactions,PCRisanexpo-nentialprocessandthereforeverysmallchangesinamplicationeciency,E,canresultindramaticdierencesintheamountofnalproduct,eveniftheinitialnumberoftargetmoleculesisthesame.
Forexample,ifE74:7%(e.
g.
,PfuTurbo,3.
9-kbFig.
3.
Real-timePCRamplicationinthepresenceofvaryingDMSOamounts.
PfuTurboDNApolymerasewasusedtoamplifythe545-bpampliconwith78%CGcontentinthepresenceofdierentamountsofDMSO(0–15%(v/v),in1%increments)(seeMaterialsandmethods).
Table4Amplicationeciencies(%)asafunctionofGCcontentPolymeraseGCcontent45%78%aPfu77.
21.
851.
31.
6PfuTurbo79.
91.
655.
21.
8PfuTurboHotstart75.
11.
154.
51.
9PfuUltra70.
81.
944.
11.
8PlatinumPfx61.
21.
128.
70.
7bTgo56.
91.
9N/ASureStartTaq78.
71.
542.
10.
4PlatinumTaq78.
50.
543.
30.
5Herculase79.
71.
154.
71.
3HerculaseHotstart80.
41.
254.
50.
8Amplicationecienciesaretheaveragesobtainedfromatleastthreeindependentexperimentswiththestandarddeviationsindicated.
Betweenfourandsixserialtemplatedilutionswereusedineachexperiment(eachdilutionwaspreparedintriplicateorquadruplicate).
N/A,nodataavailable(generationofsmearormultipleproducts).
a8%DMSOwasusedintheamplicationofthistarget.
bPCRxsolutionwasaddedaccordingtothemanufacturersrecommendation.
232B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235fragment)andn30,thenNN010:74730or1.
86107N0.
Inotherwords,after30cycles,thisPCRwouldtheoreticallyproducea1.
86107-foldincreaseintheamountoftargetmolecules.
However,ifE49:1%(e.
g.
,Pfu,3.
9-kbfragment),after30cycles,thetargetwouldbeampliedonly1.
6105timesbyPCR.
Thusa25.
6%dierenceinamplicatione-ciencyleadstoa116-folddierenceintheamountofnalproduct.
PCRproductyieldisgenerallythemostimportantparameterconsideredwhenselectingaPCRenzymeforamplication.
Despiteitsimportance,verylittlecom-parativeinformationexistswithregardtoamplicationecienciesofcommercialPCRenzymes.
Inthisstudy,wedeterminedtheamplicationeciencyof10dierentDNApolymeraseformulationsunderoptimalcondi-tions(enzymeamount,PCRbuer,extensiontempera-ture)usingidenticalreactionparameters(primerandtemplateconcentrations,cyclingregimen).
SignicantdierencesinthePCRenzymeeciencywereapparentincarefullycontrolledcomparisonsemployingvetemplatesofvaryinglengthandGCcontent.
AllDNApolymerasesexaminedexhibitedroughlysimilareciencieswhenamplifyingsmallerfragments(1–2kb)orGC-richamplicons.
Forexample,Table5showsthenumberofcyclesrequiredtoachieve106-foldamplicationusingtheeciencyvaluesdeter-B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235233minedforthe545-(Table4)and2.
6-kb(Table3)am-plicons.
AlthoughallDNApolymerasescanamplifythelow%-GCamplicons106-foldwithin30cycles,thede-siredlevelofamplicationisachieved1to7cyclesearlier,dependingontheDNApolymeraseemployed.
Forexample,the2.
6-kbampliconcanbeamplied106-foldin23cyclesusingPfuTurbo,PfuUltra,andHercu-laseDNApolymerases,comparedto29cyclesusingSureStartTaqDNApolymerase.
However,dependingonthetargetDNAsequence,theminimumnumberofcyclesrequiredtoachieve106-foldamplicationmaygreatlyexceed30cycles.
Forexample,dependingontheDNApolymeraseemployed,anadditional7to26cyclesisrequiredtoamplifythe78%GCampliconcomparedtothe45%GCamplicon(Table5).
ThehigherthenumberofPCRcycles,thehigherthechancesofam-plifyingundesiredproducts,suchasprimerdimers.
Inadditiontoeciency,PCRenzymedelityisanotherimportantconsiderationwhenamplifyinglongtargets(>1kb),sincethepercentageofclonescontainingerrorsincreasesproportionallywithincreasingampliconsize.
AsshowninTable5,Pfu+dUTPaseformulations(PfuUltra,PfuTurbo)areexpectedtoamplifylongertargetswithboththefewestnumberofcyclesandthefewestpolymerase-inducederrors.
AnumberofmodicationstothebasicPCRformatincludingadditivessuchasformamide[23],DMSO[24,25],betaine[26],etc.
havebeenpublishedinanat-tempttoincreaseamplicationeciencyandspecicity,regardlessofampliconlengthorcomposition.
Real-timePCRmethods,suchasthosedescribedinthisreport,representapowerfultoolformonitoringeortstoop-timizeamplicationeciency.
ThedatageneratedbythisprotocolarecollectedattheexponentialphaseofPCRandthereforedemonstratehighreproducibilitycomparedtoendpointanalysisbygelelectrophoresis.
QuantitativemethodsshowpromiseinthedevelopmentandqualitycontrolofPCRenzyme/buerformulationstoensureconsistencyandmaximalperformance.
AcknowledgmentsTheauthorsthankDrs.
VanessaGurtu,MadhushreeGhosh,andReinholdMuellerforcriticalreadingofthismanuscript.
References[1]K.
Mullis,F.
Faloona,S.
Scharf,R.
Saiki,G.
Horn,H.
Erlich,SpecicenzymaticamplicationofDNAinvitro:thepolymerasechainreaction,ColdSpringHarb.
Symp.
Quant.
Biol.
51(1)(1986)263–273.
[2]S.
A.
Bustin,AbsolutequanticationofmRNAusingreal-timereversetranscriptionpolymerasechainreactionassays,J.
Mol.
Endocrinol.
25(2000)169–193.
[3]R.
S.
Cha,W.
G.
Thilly,Specicity,eciency,anddelityofPCR,in:C.
W.
Dieenbach,G.
S.
Dveksler(Eds.
),PCRPrimer:ALaboratoryManual,ColdSpringHarborLaboratoryPress,ColdSpringHarbor,NY,1995.
[4]R.
J.
Wiesner,DirectquanticationofpicomolarconcentrationsofmRNAsbymathematicalanalysisofareversetranscription/exponentialpolymerasechainreactionassay,NucleicAcidsRes.
20(1992)5863–5864.
[5]R.
Higuchi,C.
Fockler,G.
Dollinger,R.
Watson,KineticPCRanalysis:real-timemonitoringofDNAamplicationreactions,Biotechnology11(1993)1026–1030.
[6]L.
L.
Ling,P.
Keohavong,C.
Dias,W.
G.
Thilly,Optimizationofthepolymerasechainreactionwithregardtodelity:modiedT7,Taq,andventDNApolymerases,PCRMethodsAppl.
1(1991)63–69.
[7]A.
M.
Dunning,P.
Talmud,S.
E.
Humphries,Errorsinthepolymerasechainreaction,NucleicAcidsRes.
16(1988)10393.
[8]P.
Keohavong,W.
G.
Thilly,FidelityofDNApolymerasesinDNAamplication,Proc.
Natl.
Acad.
Sci.
USA86(1989)9253–9257.
[9]A.
Karsai,S.
Muller,S.
Platz,M.
T.
Hauser,EvaluationofahomemadeSYBRgreenIreactionmixtureforreal-timePCRTable5VariationofcyclenumberandmutationfrequencywithDNApolymeraseDNApolymeraseErrorrate(mutationperbpperduplication)a545-bpamplicon2.
6-kbampliconPCR-inducedmutantfraction(%)bNumberofcyclesrequiredcPCR-inducedmutantfraction(%)bNumberofcyclesrequiredc45%GC78%GC+additivesPfu1.
310612433726PfuTurbo1.
310612431723PfuUltra4.
31070.
52638223Pfx3.
51064295518NAHerculase2.
8106324321523SureStartTaq8.
0106924394229aFromHogrefeandBorns[20].
bFractionoferror-containingproductsfollowing106-foldamplicationoftheindicatedtargetsequencegiventheDNApolymeraseerrorrate.
MutationfrequencieswerecalculatedusingtheequationmfERbpd,wheremfisthemutationfrequency,ERistheerrorrate,bpisthelengthofthetarget,anddisthenumberoftemplatedoublings[13].
cNumberofcyclesrequiredtoobtain106-foldamplicationgiventheeciencypercycleinTables3and5.
234B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235quanticationofgeneexpression,Biotechniques32(2002)790–792,794–796.
[10]K.
S.
Lundberg,D.
D.
Shoemaker,M.
W.
Adams,J.
M.
Short,J.
A.
Sorge,E.
J.
Mathur,High-delityamplicationusingathermo-stableDNApolymeraseisolatedfromPyrococcusfuriosus,Gene108(1991)1–6.
[11]J.
M.
Flaman,T.
Frebourg,V.
Moreau,F.
Charbonnier,C.
Martin,C.
Ishioka,S.
H.
Friend,R.
Iggo,ArapidPCRdelityassay,NucleicAcidsRes.
22(1994)3259–3260.
[12]W.
M.
Barnes,PCRamplicationofupto35-kbDNAwithhighdelityandhighyieldfromlambdabacteriophagetemplates,Proc.
Natl.
Acad.
Sci.
USA91(1994)2216–2220.
[13]J.
Cline,J.
C.
Braman,H.
H.
Hogrefe,PCRdelityofpfuDNApolymeraseandotherthermostableDNApolymerases,NucleicAcidsRes.
24(1996)3546–3551.
[14]D.
E.
Kellogg,I.
Rybalkin,S.
Chen,N.
Mukhamedova,T.
Vlasik,P.
D.
Siebert,A.
Chenchik,TaqStartAntibody:''hotstart''PCRfacilitatedbyaneutralizingmonoclonalantibodydirectedagainstTaqDNApolymerase,Biotechniques16(1994)1134–1137.
[15]H.
Mizuguchi,M.
Nakatsuji,S.
Fujiwara,M.
Takagi,T.
Imanaka,CharacterizationandapplicationtohotstartPCRofneutralizingmonoclonalantibodiesagainstKODDNApolymer-ase,J.
Biochem.
(Tokyo)126(1999)762–768.
[16]T.
Moretti,B.
Koons,B.
Budowle,EnhancementofPCRamplicationyieldandspecicityusingAmpliTaqGoldDNApolymerase,Biotechniques25(1998)716–722.
[17]M.
A.
Greagg,M.
J.
Fogg,G.
Panayotou,S.
J.
Evans,B.
A.
Connolly,L.
H.
Pearl,Aread-aheadfunctioninarchaealDNApolymerasesdetectspromutagenictemplate-stranduracil,Proc.
Natl.
Acad.
Sci.
USA96(1999)9045–9050.
[18]H.
H.
Hogrefe,C.
J.
Hansen,B.
R.
Scott,K.
B.
Nielson,ArchaealdUTPaseenhancesPCRamplicationswitharchaealDNApolymerasesbypreventingdUTPincorporation,Proc.
Natl.
Acad.
Sci.
USA99(2002)596–601.
[19]M.
Takagi,M.
Nishioka,H.
Kakihara,M.
Kitabayashi,H.
Inoue,B.
Kawakami,M.
Oka,T.
Imanaka,CharacterizationofDNApolymerasefromPyrococcussp.
strainKOD1anditsapplicationtoPCR,Appl.
Environ.
Microbiol.
63(1997)4504–4510.
[20]H.
H.
Hogrefe,M.
Borns,HighdelityPCRenzymes,in:C.
W.
Dieenbach,G.
S.
Dveksler(Eds.
),PCRPrimer:ALaboratoryManual,ColdSpringHarborLaboratoryPress,ColdSpringHarbor,NY,2003.
[21]H.
H.
Hogrefe,J.
Cline,A.
E.
Lovejoy,K.
B.
Nielson,DNApolymerasesfromhyperthermophiles,MethodsEnzymol.
334(2001)91–116.
[22]W.
A.
Al-Soud,P.
Radstrom,PuricationandcharacterizationofPCR-inhibitorycomponentsinbloodcells,J.
Clin.
Microbiol.
39(2001)485–493.
[23]G.
Sarkar,S.
Kapelner,S.
S.
Sommer,Formamidecandramat-icallyimprovethespecicityofPCR,NucleicAcidsRes.
18(1990)7465.
[24]P.
R.
Winship,AnimprovedmethodfordirectlysequencingPCRampliedmaterialusingdimethylsulphoxide,NucleicAcidsRes.
17(1989)1266.
[25]R.
Chakrabarti,C.
E.
Schutt,NovelsulfoxidesfacilitateGC-richtemplateamplication,Biotechniques32(2002)866,868,870–872,874.
[26]W.
Henke,K.
Herdel,K.
Jung,D.
Schnorr,S.
A.
Loening,BetaineimprovesthePCRamplicationofGC-richDNAsequences,NucleicAcidsRes.
25(1997)3957–3958.
B.
Arezietal.
/AnalyticalBiochemistry321(2003)226–235235
特网云(198元/月),高质量云虚拟主机低至0.16元/天,裸金属服务器仅需10.5元/天
特网云为您提供高速、稳定、安全、弹性的云计算服务计算、存储、监控、安全,完善的云产品满足您的一切所需,深耕云计算领域10余年;我们拥有前沿的核心技术,始终致力于为政府机构、企业组织和个人开发者提供稳定、安全、可靠、高性价比的云计算产品与服务。官方网站:https://www.56dr.com/ 10年老品牌 值得信赖 有需要的请联系======================特网云推出多IP云主机...
Kinponet是谁?Kinponet前身公司叫金宝idc 成立于2013年 开始代理销售美国vps。
在2014年发现原来使用VPS的客户需求慢慢的在改版,VPS已经不能满足客户的需求。我们开始代理机房的独立服务器,主推和HS机房的独立服务器。经过一年多的发展,我们发现代理的服务器配置参差不齐,机房的售后服务也无法完全跟上,导致了很多问题发生,对使用体验带来了很多的不便,很多客户离开了我们。经过我们慎重的考虑和客户的建议。我们在2015开始了重大的改变, 2015年,我们开始计划托管自己...
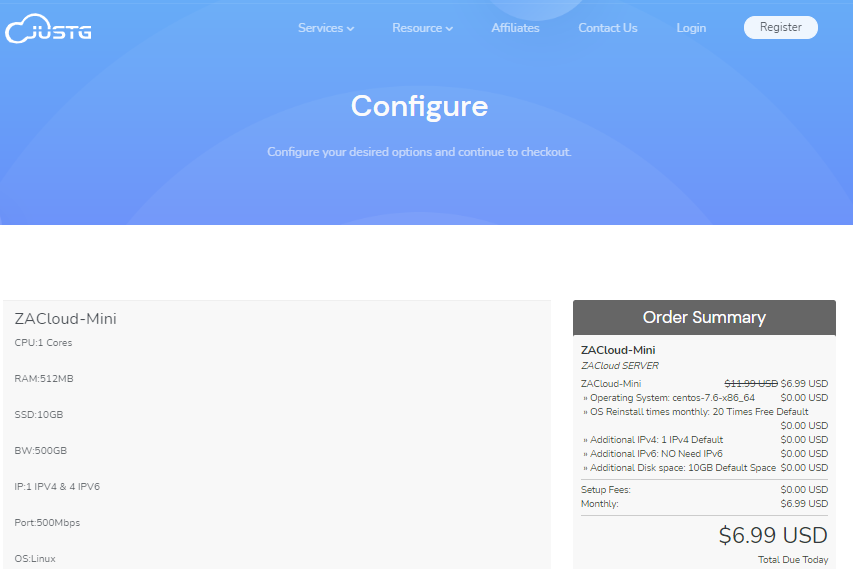
JUSTG(5.99美元/月)最新5折优惠,KVM虚拟虚拟512Mkvm路线
Justg是一家俄罗斯VPS云服务器提供商,主要提供南非地区的VPS服务器产品,CN2高质量线路网络,100Mbps带宽,自带一个IPv4和8个IPv6,线路质量还不错,主要是用户较少,带宽使用率不高,比较空闲,不拥挤,比较适合面向非洲、欧美的用户业务需求,也适合追求速度快又需要冷门的朋友。justg的俄罗斯VPS云服务器位于莫斯科机房,到美国和中国速度都非常不错,到欧洲的平均延迟时间为40毫秒,...
wle为你推荐
-
苏州商标注册在江苏怎么注册商标啊??快递打印如何快递打印快递单96155北京住房公积金电话96155经常没人接?绵阳电信绵阳电信宽带资费渗透测试web渗透测试有前途吗唱吧电脑版官方下载唱吧有没有电脑版的啊?腾讯文章腾讯罗剑楠是何许人也?人人逛街包公免费逛街打一成语bluestack安卓模拟器bluestacks怎么用?如何清理ie缓存怎么清理IE的缓存