iiu998
u998 时间:2021-03-01 阅读:()
ExtratelomericbindingofTRF1andTRF21028npgCellResearch|Vol21No7|July2011ORIGINALARTICLEThehumanTTAGGGrepeatfactors1and2bindtoasubsetofinterstitialtelomericsequencesandsatelliterepeatsThomasSimonet1,Laure-EmmanuelleZaragosi2,ClaudePhilippe3,KevinLebrigand2,ClémentineSchouteden1,AdelineAugereau1,3,SergeBauwens1,JingYe1,3,MarcoSantagostino4,ElenaGiulotto4,FrederiqueMagdinier1,BéatriceHorard1,PascalBarbry2,RainerWaldmann2,EricGilson1,3,51LaboratoiredeBiologieMoléculairedelaCellule-UMR5239CNRS/ENSLyon/UniversitéLyon,EcoleNormaleSupérieuredeLyon,46alléed'Italie,Lyon69364,France;2CNRSandUniversityofNiceSophiaAntipolis,InstitutdePharmacologieMolé-culaireetCellulaire,06560SophiaAntipolis,France;3LaboratoryofBiologyandPathologyofGenomesofUniversityofNiceSophia-Antipolis,CNRSUMR6267/INSERMU998,FacultyofMedicine,Nice,France;4DipartimentodiGeneticaeMicrobiologiaAdrianoBuzzati-Traverso,UniversitàdiPavia,Pavia,Italy;5DepartmentofMedicalGenetics,CHUofNice,Nice,FranceCorrespondence:EricGilsonTel:+33-472728453;Fax:+33-472728080E-mail:Eric.
Gilson@unice.
frReceived3November2010;revised9January2011;accepted11January2011;publishedonline22March2011ThestudyoftheproteinsthatbindtotelomericDNAinmammalshasprovidedadeepunderstandingofthemech-anismsinvolvedinchromosome-endprotection.
However,verylittleisknownonthebindingoftheseproteinstonontelomericDNAsequences.
TheTTAGGGDNArepeatproteins1and2(TRF1andTRF2)bindtomammaliante-lomeresaspartoftheshelterincomplexandareessentialformaintainingchromosomeendstability.
Inthisstudy,wecombinedchromatinimmunoprecipitationwithhigh-throughputsequencingtomapathighsensitivityandresolutionthehumanchromosomalsitestowhichTRF1andTRF2bind.
Whilemostoftheidentifiedsequencescorrespondtotelomericregions,weshowedthatthesetwoproteinsalsobindtoextratelomericsites.
Thevastmajorityoftheseex-tratelomericsitescontainsinterstitialtelomericsequences(orITSs).
However,wealsoidentifiednon-ITSsites,whichcorrespondtocentromericandpericentromericsatelliteDNA.
Interestingly,theTRF-bindingsitesareoftenlocatedintheproximityofgenesorwithinintrons.
WeproposethatTRF1andTRF2couplethefunctionalstateoftelomerestothelong-rangeorganizationofchromosomesandgeneregulationnetworksbybindingtoextratelomericsequences.
Keywords:telomere;TRF1;TRF2;interstitialtelomericsequence;satelliteDNACellResearch(2011)21:1028-1038.
doi:10.
1038/cr.
2011.
40;publishedonline22March2011npgCellResearch(2011)21:1028-1038.
2011IBCB,SIBS,CASAllrightsreserved1001-0602/11$32.
00www.
nature.
com/crIntroductionTheparamountimportanceoftelomerestocellfatelikelystemsfromthegreatdiversityinthefunctionstheyperform[1,2].
Theycontrolthereplicationofchro-mosomalDNAtermini,protectchromosomeendsfromDNArepairandcheckpointactivation,controlthemei-oticspindle,localizethechromosomeendswithinthenuclearspaceandregulatelong-rangechromatinchangesaswellasgeneexpression.
Telomeresconsistofspecificnucleoproteincomplexes[3].
TelomericDNAhassev-eraldistinctivefeatures,includingasequenceformedbyrepetitionsofasmallG-richmotif(TTAGGGinmam-mals)andthepresenceofasingle-strandedtailonthe3′-orientedstrand(Gtail).
TelomericDNAistranscribedintoaUUAGGGrepeat-containingRNAcalledTERRA,whichisbelievedtoplayfundamentalrolesintelomerebiology[4,5].
Akeycomponentofthemammaliantelomereistheshelterincomplex,whichiscomposedofsixpolypep-tides:TRF1,TRF2,Rap1,Tin2,TPP1andPot1[5].
Ofthese,threebindspecificallytoTTAGGGrepeats:TRF1andTRF2,whichrecognizetheduplexDNA,andPot1,whichbindstothesingle-stranded3′overhangs[3,6].
TRF1andTRF2donotexistinbuddingyeast.
Instead,yeastRap1actsasanessentialcappingfactorthatbindstotelomericDNA,whileyeastCdc13bindstothe3′overhangandseemstoperformfunctionsthataresimilartothoseofPot1andTPP1[7].
Telomeresinyeastandmammalscansilenceneigh-www.
cell-research.
com|CellResearchThomasSimonetetal.
1029npgboringgenesbyexertingtelomericpositioneffect(orTPE)[8-10].
TPEisinfluencedbytelomerelengthandstructureaswellasbychromatin-remodelingmachiner-ies[11].
Telomericandsubtelomericchromatindifferfromconstitutiveheterochromatinintermsofstructureanddynamics,specificityofDNAsequences,andbind-ingofspecificfactors[12].
Themechanismsthatinitiatetheformationofheterochromatinattelomeresareun-knownbutlikelyinvolvethebindingofspecificfactorstotelomericDNA.
Forinstance,theN-terminalpartofTRF2mayfacilitateheterochromatinformationbybind-ingtoORC1andTERRA[13].
RepetitionsoftheTTAGGGtelomericunit,calledinterstitialtelomericsequences,orITSs,arealsopresentwithinchromosomes[14].
Inhumans,threeclassesofITSswereidentified[15]:(i)subtelomericITSs,locatedwithinsubtelomericdomainsandcomposedofextendedarrays(usuallyseveralhundredsofbasepairs),includingmanydegenerateunits;theyprobablyarosefromrecom-binationeventsinvolvingchromosometermini[16];(ii)shortinternalITSs,locatedawayfromtelomeresandcomposedofrelativelyfewTTAGGGunits;theseITSsarelikelytohavebeengeneratedduringtherepairofDNAdouble-strandbreaksthatoccurredduringevolu-tion[17];(iii)onefusionITS,locatedin2q14,derivedfromtheendfusionbetweenthetwoancestralchromo-somesthatgaverisetohumanchromosome2[18].
NoclearindicationofanyparticularfunctionofITSshasbeenprovidedsofar.
Emergingevidenceindicatesthattheshelterincom-ponentshavenon-telomericfunctionsinDNArepair[19],Epstein-Barrvirusreplication[20],transcriptionalregulation[21]andNF-κBactivation[22].
Thesenon-telomericfunctionsmightbe,atleastpartially,explainedbytheirbindingtoITSs.
Indeed,thereismountingindi-cationthatshelterincomponentscanbindtointerstitialDNAsequences:(i)TRF1andTRF2bindtotheperi-centromericregionsofhamsterchromosomescontaininglargeblocksofITSs[23,24];(ii)TRF2andTIN2bindtoanITSformedbyararehumanchromosomerear-rangement[25];(iii)TRF2bindstoastretchoftelomericsequencethatisartificiallyinsertedinthemiddleofthelongarmofchromosome4[26];(iv)Rap1bindstoseveralITSsofthemousegenome[27].
However,threenaturallyoccurringITSsofhumanchromosomesdonotappeartobeboundbyTRF2[26].
Therefore,itisstillunclearwhetherTRF1andTRF2reallybindtotheITSsnormallyfoundinhumanchromosomesoreventounre-latedsequences.
Moreover,thereisevidencethatTRF2modulatesgeneexpressionoutsidefromtelomeressinceitinteractswiththerepressorelement1-silencingtran-scriptionfactor(REST),arepressorofgenesdevotedtoneuronalfunctions[21].
Inthisstudy,wemappedthehumanchromosomalsitestowhichTRF1andTRF2bindbycombiningchro-matinimmunoprecipitationwithhigh-throughputDNAsequencing(ChIP-Seq).
ResultsIdentificationofTRFbindingsitesbyChIP-SeqanalysisToestablishglobalbindingprofilesofTRF1andTRF2(collectivelynamedtheTRFproteins),weperformedaChIP-SeqanalysiswithoneantibodyspecificforTRF1andtwoantibodiesspecificforTRF2(onemonoclonalorTRF2m,onepolyclonalorTRF2p).
WeusedtheBJ-HELTRasmctumorcelllinebecauseTRF2isrequiredfortumorigenicitythroughapathwaythatinvolvesuncou-plingoftelomereprotectionandtheDNAdamagere-sponsemechanism,suggestingaroleforextratelomericTRF2bindingsitesinoncogenesis(Biroccioetal,sub-mitted).
Thespecificityoftheanti-TRF1andanti-TRF2antibodieswasconfirmedbyslotblotanalysis(Figure1A).
Wefoundupto50-foldenrichmentoftelomericsequencesintheTRFantibody-immunoprecipitatedsam-pleswhencomparedtoProteinG-Sepharose-precipitatedcontrolsamplesandtotalhistoneH3-immunoprecipi-tation.
ThisresultwasconfirmedbytheanalysisoftheChIP-Seqreads.
InTRFantibody-immunoprecipitatedsampleswedetected90to150timesmoresequencesthatcontainsolelythe(TTAGGG)nmotifthaninthecontrolsamples(Figure1B).
ToidentifyextratelomericbindingsitesfortheTRFproteins,weretainedonlyreadsthatwereuniquelyalignedonthe2006Humangenomeassembly(NCBI36/hg18),andwecheckedthatpure(TTAGGG)nreads,whichlikelyoriginatefromtelomericDNA,hadbeenindeedcompletelydiscarded.
Significantlyread-enrichedpositionsorpeakswereidentifiedusingtheSISSRsoftware[28]withaPvaluethresholdof0.
001usingproteinGimmunoprecipitationasbackground.
Wefur-therremovedtheseeminglyartifactual(non-specific)peaksthroughavisualinspectionofadensityprofileofthematchedreads(seetheexampleforchromosome1,showninSupplementaryinformation,FigureS1).
Fol-lowingthisfiltering,weidentified68peakspresentinallthreeTRFChIP-Seqsamples(TRF1,TRF2mandTRF2p)(Figure2A).
Resultsforchromosome1areshowninFigure2BandthoseforotherchromosomesareshowninSupplementaryinformation,FigureS2.
Notably,18peaksfromtheTRF2mChIP(amongn=90,20%)werenotfoundusingTRF2pantibody,while21peaksidentifiedbytheTRF2pChIP(n=93,22.
5%)werenotpresentinTRF2mChIP.
FormostofExtratelomericbindingofTRF1andTRF21030npgCellResearch|Vol21No7|July2011Figure1(A)SlotblotshowingthetelomericenrichmentofDNAimmunoprecipitatedwithanti-TRF1orTRF2antibodies.
DNAimmunoprecipitatedbyatotalH3antibodyandpulleddownbyproteinGalonewasusedasacontrol.
HalfoftheprecipitatedDNAwasloaded,alongwithaninputscale(2500ngto10ng,correspondingto10%to0.
04%ofthetotalinput),andhybrid-izedsequentiallytoatelomericprobeandagenomicprobe.
Foreachprobe,wequantifiedthefractionoftheimmunoprecipi-tatedDNA.
Theratioofthevalueobtainedforthetelomericprobetothegenomicprobeisthetelomericenrichmentfactor.
(B)Foldenrichmentofthefractionofrawreadscontainingonly(TTAGGG)nsequencesfromTRFChIP-SeqasnormalizedtothereadsobtainedthroughimmunoprecipitationofproteinG.
Figure2(A)TRF1,TRF2m,andTRF2pChIP-Seqpeaks.
Thepeakslargelycoincide,asshownontheVenndiagram.
As-sessmentofoverlapswasperformedbyvisualinspectionintheIntegratedGenomeBrowser.
(B)VisualizationofTRFpeaksandTRFbindingsites.
Regionsofsignificantreadenrichment(PU998)forcriticalreading.
WearealsogratefultoZhouSongyang(BaylorCollegeofMedicine)forsharingunpublishedresults.
ThisworkwassupportedbygrantsfromtheAssociationdelarecherchecontreleCancer(ARC),theInstitutNationalduCancer(programTELOFUN),ANR(programTELOREPandINNATELO)andtheEuropeanCommunity(TELOMARKERHealth-F2-2007-200950).
TSandLEZthanktheFondationdelaRechercheMédicale(FRM)andtheARC,respectively,fortheirfellowships.
References1BlackburnEH.
Telomerestatesandcellfates.
Nature2000;408:53-56.
2Segal-BendirdjianE,GilsonE.
Telomeresandtelomerase:frombasicresearchtoclinicalapplications.
Biochimie2008;90:1-4.
3Giraud-PanisMJ,PisanoS,PouletA,LeDuMH,GilsonE.
Structuralidentityoftelomericcomplexes.
FEBSLett2010;584:3785-3799.
4AzzalinCM,ReichenbackP,KhoriauliL,GiulottoE,LingnerJ.
TelomericrepeatcontainingRNAandRNAsurveillancefactorsatmammalianchromosomeends.
Science2007;318:798-801.
5SchoeftnerS,BlascoMA.
Developmentallyregulatedtran-scriptionofmammaliantelomeresbyDNA-dependentRNApolymeraseII.
NatCellBiol2008;10:228-236.
6CelliGB,deLangeT.
DNAprocessingisnotrequiredforATM-mediatedtelomeredamageresponseafterTRF2dele-tion.
NatCellBiol2005;7:712-718.
7Giraud-PanisMJ,TeixeiraMT,GeliV,GilsonE.
CSTmeetsshelterintokeeptelomeresincheck.
MolCell2010;39:665-676.
8GottschlingDE,AparicioOM,BillingtonBL,ZakianVA.
Po-sitioneffectatS.
cerevisiaetelomeres:reversiblerepresssionofPolIItranscription.
Cell1990;63:751-762.
9BaurJA,ZouY,ShayJW,WrightWE.
Telomerepositionef-fectinhumancells.
Science2001;292:2075-2077.
10KoeringCE,PolliceA,ZibellaMP,etal.
Humantelomericpositioneffectisdeterminedbychromosomalcontextandte-lomericchromatinintegrity.
EMBORep2002;3:1055-1061.
11OttavianiA,GilsonE,MagdinierF.
Telomericpositioneffect:fromtheyeastparadigmtohumanpathologiesBiochimie2008;90:93-107.
12BlascoMA.
Theepigeneticregulationofmammaliantelom-eres.
NatRevGenet2007;8:299-309.
13DengZ,NorseenJ,WiedmerA,RiethmanH,LiebermanPM.
TERRARNAbindingtoTRF2facilitatesheterochromatinformationandORCrecruitmentattelomeres.
MolCell2009;35:403-413.
14Ruiz-HerreraA,NergadzeSG,SantagostinoM,GiulottoE.
Telomericrepeatsfarfromtheends:mechanismsoforiginandroleinevolution.
CytogenetGenomeRes2008;122:219-228.
15AzzalinCM,NergadzeSG,GiulottoE.
Humanintrachro-mosomaltelomeric-likerepeats:sequenceorganizationandmechanismsoforigin.
Chromosoma2001;110:75-82.
16AmbrosiniA,PaulS,HuS,RiethmanH.
Humansubtelomer-icdupliconstructureandorganization.
GenomeBiol2007;8:R151.
17NergadzeSG,SantagostinoMA,SalzanoA,MondelloC,GiulottoE.
ContributionoftelomeraseRNAretrotranscrip-tiontoDNAdouble-strandbreakrepairduringmammaliangenomeevolution.
GenomeBiol2007;8:R260.
18IjdoJW,BaldiniA,WardDC,ReedersST,WellsRA.
Originofhumanchromosome2:anancestraltelomere-telomerefu-sion.
ProcNatlAcadSciUSA1991;88:9051-9055.
19BradshawPS,StavropoulosDJ,MeynMS.
Humantelo-mericproteinTRF2associateswithgenomicdouble-strandbreaksasanearlyresponsetoDNAdamage.
NatGenet2005;37:193-197.
20DengZ,LezinaL,ChenCJ,etal.
TelomericproteinsregulateepisomalmaintenanceofEpstein-Barrvirusoriginofplasmidreplication.
MolCell2002;9:493-503.
21ZhangP,PazinMJ,SchwartzCM,etal.
NontelomericTRF2-RESTinteractionmodulatesneuronalgenesilencingandfateoftumorandstemcells.
CurrBiol2008;18:1489-1494.
22TeoH,GhoshS,LueschH,etal.
Telomere-independentRap1isanIKKadaptorandregulatesNF-kappaB-dependentgeneexpression.
NatCellBiol2010;12:758-767.
23SmogorzewskaA,vanSteenselB,BianchiA,etal.
ControlofhumantelomerelengthbyTRF1andTRF2.
MolCellBiol2000;20:1659-1668.
24KrutilinaRI,SmirnovaAN,MudrakOS,etal.
Protectionofinternal(TTAGGG)nrepeatsinChinesehamstercellsbytelo-mericproteinTRF1.
Oncogene2003;22:6690-6698.
25Mignon-RavixC,DepetrisD,DelobelB,CroquetteMF,Mat-teiMG.
AhumaninterstitialtelomereassociatesinvivowithspecificTRF2andTIN2proteins.
EurJHumGenet2002;10:107-112.
26YeJ,LenainC,BauwensS,etal.
TRF2andapollocooperatewithtopoisomerase2alphatoprotecthumantelomeresfromreplicativedamage.
Cell2010;142:230-242.
27MartinezP,ThanasoulaM,CarlosAR,etal.
MammalianRap1controlstelomerefunctionandgeneexpressionthroughbindingtotelomericandextratelomericsites.
NatCellBiol2010;12:768-780.
28JothiR,CuddapahS,BarskiA,CuiK,ZhaoK.
Genome-wideidentificationofinvivoprotein-DNAbindingsitesfromChIP-Seqdata.
NucleicAcidsRes2008;36:5221-5231.
29EdgarR,DomrachevM,LashAE.
GeneExpressionOmni-bus:NCBIgeneexpressionandhybridizationarraydatare-pository.
NucleicAcidsRes2002;30:207-210.
30DesmazeC,AlbertiC,MartinsL,etal.
Theinfluenceofin-terstitialtelomericsequencesonchromosomeinstabilityinhumancells.
CytogenetCellGenet1999;86:288-295.
31MondelloC,PirzioL,AzzalinCM,GiulottoE.
Instabilityofinterstitialtelomericsequencesinthehumangenome.
Ge-nomics2000;68:111-117.
32LeeC,WevrickR,FisherRB,Ferguson-SmithMA,LinCC.
HumancentromericDNAs.
HumGenet1997;100:291-304.
ExtratelomericbindingofTRF1andTRF21038npgCellResearch|Vol21No7|July201133JohnsonDS,MortazaviA,MyersRM,WoldB.
Genome-widemappingofinvivoprotein-DNAinteractions.
Science2007;316:1497-1502.
34YangD,XiongY,KimH,etal.
Humantelomericproteinsoccupyselectiveinterstitialsites.
CellRes2011Mar22.
doi:10.
1038/cr.
2011.
3935SfeirA,KosiyatrakulST,HockemeyerD,etal.
MammaliantelomeresresemblefragilesitesandrequireTRF1forefficientreplication.
Cell2009;138:90-103.
36MartínezP,ThanasoulaM,MuozP,etal.
IncreasedtelomerefragilityandfusionsresultingfromTRF1deficienciesleadtodegenerativepathologiesandincreasedcancerinmice.
GenesDev2009;23:2060-2075.
37MailletL,BoscheronC,GottaM,etal.
Evidenceforsilenc-ingcompartmentswithintheyeastnucleus:arolefortelomereproximityandSir-proteinconcentrationinsilencer-mediatedrepression.
GenesDev1996;10:1796-1811.
38MarcandS,BuckSW,MorettiP,GilsonE,ShoreD.
Silenc-ingofgenesatnontelomericsitesinyeastiscontrolledbyse-questrationofsilencingfactorsattelomeresbyRap1protein.
GenesDev1996;10:1297-1309.
39BaileyTL,ElkanC.
Fittingamixturemodelbyexpectationmaximizationtodiscovermotifsinbiopolymers.
ProcIntConfIntellSystMolBiol1994;2:28-36.
40BlahnikKR,DouL,O'GeenH,etal.
Sole-Search:aninte-gratedanalysisprogramforpeakdetectionandfunctionalannotationusingChIP-seqdata.
NucleicAcidsRes2010;38:e13.
41JurkaJ,KapitonovVV,PavlicekA,etal.
RepbaseUpdate,adatabaseofeukaryoticrepetitiveelements.
CytogenetGenomeRes2005;110:462-467.
42HuangdaW,ShermanBT,LempickiRA.
SystematicandintegrativeanalysisoflargegenelistsusingDAVIDbioinfor-maticsresources.
NatProtoc2009;4:44-57.
(SupplementaryinformationislinkedtotheonlineversionofthepaperontheCellResearchwebsite.
)
Gilson@unice.
frReceived3November2010;revised9January2011;accepted11January2011;publishedonline22March2011ThestudyoftheproteinsthatbindtotelomericDNAinmammalshasprovidedadeepunderstandingofthemech-anismsinvolvedinchromosome-endprotection.
However,verylittleisknownonthebindingoftheseproteinstonontelomericDNAsequences.
TheTTAGGGDNArepeatproteins1and2(TRF1andTRF2)bindtomammaliante-lomeresaspartoftheshelterincomplexandareessentialformaintainingchromosomeendstability.
Inthisstudy,wecombinedchromatinimmunoprecipitationwithhigh-throughputsequencingtomapathighsensitivityandresolutionthehumanchromosomalsitestowhichTRF1andTRF2bind.
Whilemostoftheidentifiedsequencescorrespondtotelomericregions,weshowedthatthesetwoproteinsalsobindtoextratelomericsites.
Thevastmajorityoftheseex-tratelomericsitescontainsinterstitialtelomericsequences(orITSs).
However,wealsoidentifiednon-ITSsites,whichcorrespondtocentromericandpericentromericsatelliteDNA.
Interestingly,theTRF-bindingsitesareoftenlocatedintheproximityofgenesorwithinintrons.
WeproposethatTRF1andTRF2couplethefunctionalstateoftelomerestothelong-rangeorganizationofchromosomesandgeneregulationnetworksbybindingtoextratelomericsequences.
Keywords:telomere;TRF1;TRF2;interstitialtelomericsequence;satelliteDNACellResearch(2011)21:1028-1038.
doi:10.
1038/cr.
2011.
40;publishedonline22March2011npgCellResearch(2011)21:1028-1038.
2011IBCB,SIBS,CASAllrightsreserved1001-0602/11$32.
00www.
nature.
com/crIntroductionTheparamountimportanceoftelomerestocellfatelikelystemsfromthegreatdiversityinthefunctionstheyperform[1,2].
Theycontrolthereplicationofchro-mosomalDNAtermini,protectchromosomeendsfromDNArepairandcheckpointactivation,controlthemei-oticspindle,localizethechromosomeendswithinthenuclearspaceandregulatelong-rangechromatinchangesaswellasgeneexpression.
Telomeresconsistofspecificnucleoproteincomplexes[3].
TelomericDNAhassev-eraldistinctivefeatures,includingasequenceformedbyrepetitionsofasmallG-richmotif(TTAGGGinmam-mals)andthepresenceofasingle-strandedtailonthe3′-orientedstrand(Gtail).
TelomericDNAistranscribedintoaUUAGGGrepeat-containingRNAcalledTERRA,whichisbelievedtoplayfundamentalrolesintelomerebiology[4,5].
Akeycomponentofthemammaliantelomereistheshelterincomplex,whichiscomposedofsixpolypep-tides:TRF1,TRF2,Rap1,Tin2,TPP1andPot1[5].
Ofthese,threebindspecificallytoTTAGGGrepeats:TRF1andTRF2,whichrecognizetheduplexDNA,andPot1,whichbindstothesingle-stranded3′overhangs[3,6].
TRF1andTRF2donotexistinbuddingyeast.
Instead,yeastRap1actsasanessentialcappingfactorthatbindstotelomericDNA,whileyeastCdc13bindstothe3′overhangandseemstoperformfunctionsthataresimilartothoseofPot1andTPP1[7].
Telomeresinyeastandmammalscansilenceneigh-www.
cell-research.
com|CellResearchThomasSimonetetal.
1029npgboringgenesbyexertingtelomericpositioneffect(orTPE)[8-10].
TPEisinfluencedbytelomerelengthandstructureaswellasbychromatin-remodelingmachiner-ies[11].
Telomericandsubtelomericchromatindifferfromconstitutiveheterochromatinintermsofstructureanddynamics,specificityofDNAsequences,andbind-ingofspecificfactors[12].
Themechanismsthatinitiatetheformationofheterochromatinattelomeresareun-knownbutlikelyinvolvethebindingofspecificfactorstotelomericDNA.
Forinstance,theN-terminalpartofTRF2mayfacilitateheterochromatinformationbybind-ingtoORC1andTERRA[13].
RepetitionsoftheTTAGGGtelomericunit,calledinterstitialtelomericsequences,orITSs,arealsopresentwithinchromosomes[14].
Inhumans,threeclassesofITSswereidentified[15]:(i)subtelomericITSs,locatedwithinsubtelomericdomainsandcomposedofextendedarrays(usuallyseveralhundredsofbasepairs),includingmanydegenerateunits;theyprobablyarosefromrecom-binationeventsinvolvingchromosometermini[16];(ii)shortinternalITSs,locatedawayfromtelomeresandcomposedofrelativelyfewTTAGGGunits;theseITSsarelikelytohavebeengeneratedduringtherepairofDNAdouble-strandbreaksthatoccurredduringevolu-tion[17];(iii)onefusionITS,locatedin2q14,derivedfromtheendfusionbetweenthetwoancestralchromo-somesthatgaverisetohumanchromosome2[18].
NoclearindicationofanyparticularfunctionofITSshasbeenprovidedsofar.
Emergingevidenceindicatesthattheshelterincom-ponentshavenon-telomericfunctionsinDNArepair[19],Epstein-Barrvirusreplication[20],transcriptionalregulation[21]andNF-κBactivation[22].
Thesenon-telomericfunctionsmightbe,atleastpartially,explainedbytheirbindingtoITSs.
Indeed,thereismountingindi-cationthatshelterincomponentscanbindtointerstitialDNAsequences:(i)TRF1andTRF2bindtotheperi-centromericregionsofhamsterchromosomescontaininglargeblocksofITSs[23,24];(ii)TRF2andTIN2bindtoanITSformedbyararehumanchromosomerear-rangement[25];(iii)TRF2bindstoastretchoftelomericsequencethatisartificiallyinsertedinthemiddleofthelongarmofchromosome4[26];(iv)Rap1bindstoseveralITSsofthemousegenome[27].
However,threenaturallyoccurringITSsofhumanchromosomesdonotappeartobeboundbyTRF2[26].
Therefore,itisstillunclearwhetherTRF1andTRF2reallybindtotheITSsnormallyfoundinhumanchromosomesoreventounre-latedsequences.
Moreover,thereisevidencethatTRF2modulatesgeneexpressionoutsidefromtelomeressinceitinteractswiththerepressorelement1-silencingtran-scriptionfactor(REST),arepressorofgenesdevotedtoneuronalfunctions[21].
Inthisstudy,wemappedthehumanchromosomalsitestowhichTRF1andTRF2bindbycombiningchro-matinimmunoprecipitationwithhigh-throughputDNAsequencing(ChIP-Seq).
ResultsIdentificationofTRFbindingsitesbyChIP-SeqanalysisToestablishglobalbindingprofilesofTRF1andTRF2(collectivelynamedtheTRFproteins),weperformedaChIP-SeqanalysiswithoneantibodyspecificforTRF1andtwoantibodiesspecificforTRF2(onemonoclonalorTRF2m,onepolyclonalorTRF2p).
WeusedtheBJ-HELTRasmctumorcelllinebecauseTRF2isrequiredfortumorigenicitythroughapathwaythatinvolvesuncou-plingoftelomereprotectionandtheDNAdamagere-sponsemechanism,suggestingaroleforextratelomericTRF2bindingsitesinoncogenesis(Biroccioetal,sub-mitted).
Thespecificityoftheanti-TRF1andanti-TRF2antibodieswasconfirmedbyslotblotanalysis(Figure1A).
Wefoundupto50-foldenrichmentoftelomericsequencesintheTRFantibody-immunoprecipitatedsam-pleswhencomparedtoProteinG-Sepharose-precipitatedcontrolsamplesandtotalhistoneH3-immunoprecipi-tation.
ThisresultwasconfirmedbytheanalysisoftheChIP-Seqreads.
InTRFantibody-immunoprecipitatedsampleswedetected90to150timesmoresequencesthatcontainsolelythe(TTAGGG)nmotifthaninthecontrolsamples(Figure1B).
ToidentifyextratelomericbindingsitesfortheTRFproteins,weretainedonlyreadsthatwereuniquelyalignedonthe2006Humangenomeassembly(NCBI36/hg18),andwecheckedthatpure(TTAGGG)nreads,whichlikelyoriginatefromtelomericDNA,hadbeenindeedcompletelydiscarded.
Significantlyread-enrichedpositionsorpeakswereidentifiedusingtheSISSRsoftware[28]withaPvaluethresholdof0.
001usingproteinGimmunoprecipitationasbackground.
Wefur-therremovedtheseeminglyartifactual(non-specific)peaksthroughavisualinspectionofadensityprofileofthematchedreads(seetheexampleforchromosome1,showninSupplementaryinformation,FigureS1).
Fol-lowingthisfiltering,weidentified68peakspresentinallthreeTRFChIP-Seqsamples(TRF1,TRF2mandTRF2p)(Figure2A).
Resultsforchromosome1areshowninFigure2BandthoseforotherchromosomesareshowninSupplementaryinformation,FigureS2.
Notably,18peaksfromtheTRF2mChIP(amongn=90,20%)werenotfoundusingTRF2pantibody,while21peaksidentifiedbytheTRF2pChIP(n=93,22.
5%)werenotpresentinTRF2mChIP.
FormostofExtratelomericbindingofTRF1andTRF21030npgCellResearch|Vol21No7|July2011Figure1(A)SlotblotshowingthetelomericenrichmentofDNAimmunoprecipitatedwithanti-TRF1orTRF2antibodies.
DNAimmunoprecipitatedbyatotalH3antibodyandpulleddownbyproteinGalonewasusedasacontrol.
HalfoftheprecipitatedDNAwasloaded,alongwithaninputscale(2500ngto10ng,correspondingto10%to0.
04%ofthetotalinput),andhybrid-izedsequentiallytoatelomericprobeandagenomicprobe.
Foreachprobe,wequantifiedthefractionoftheimmunoprecipi-tatedDNA.
Theratioofthevalueobtainedforthetelomericprobetothegenomicprobeisthetelomericenrichmentfactor.
(B)Foldenrichmentofthefractionofrawreadscontainingonly(TTAGGG)nsequencesfromTRFChIP-SeqasnormalizedtothereadsobtainedthroughimmunoprecipitationofproteinG.
Figure2(A)TRF1,TRF2m,andTRF2pChIP-Seqpeaks.
Thepeakslargelycoincide,asshownontheVenndiagram.
As-sessmentofoverlapswasperformedbyvisualinspectionintheIntegratedGenomeBrowser.
(B)VisualizationofTRFpeaksandTRFbindingsites.
Regionsofsignificantreadenrichment(PU998)forcriticalreading.
WearealsogratefultoZhouSongyang(BaylorCollegeofMedicine)forsharingunpublishedresults.
ThisworkwassupportedbygrantsfromtheAssociationdelarecherchecontreleCancer(ARC),theInstitutNationalduCancer(programTELOFUN),ANR(programTELOREPandINNATELO)andtheEuropeanCommunity(TELOMARKERHealth-F2-2007-200950).
TSandLEZthanktheFondationdelaRechercheMédicale(FRM)andtheARC,respectively,fortheirfellowships.
References1BlackburnEH.
Telomerestatesandcellfates.
Nature2000;408:53-56.
2Segal-BendirdjianE,GilsonE.
Telomeresandtelomerase:frombasicresearchtoclinicalapplications.
Biochimie2008;90:1-4.
3Giraud-PanisMJ,PisanoS,PouletA,LeDuMH,GilsonE.
Structuralidentityoftelomericcomplexes.
FEBSLett2010;584:3785-3799.
4AzzalinCM,ReichenbackP,KhoriauliL,GiulottoE,LingnerJ.
TelomericrepeatcontainingRNAandRNAsurveillancefactorsatmammalianchromosomeends.
Science2007;318:798-801.
5SchoeftnerS,BlascoMA.
Developmentallyregulatedtran-scriptionofmammaliantelomeresbyDNA-dependentRNApolymeraseII.
NatCellBiol2008;10:228-236.
6CelliGB,deLangeT.
DNAprocessingisnotrequiredforATM-mediatedtelomeredamageresponseafterTRF2dele-tion.
NatCellBiol2005;7:712-718.
7Giraud-PanisMJ,TeixeiraMT,GeliV,GilsonE.
CSTmeetsshelterintokeeptelomeresincheck.
MolCell2010;39:665-676.
8GottschlingDE,AparicioOM,BillingtonBL,ZakianVA.
Po-sitioneffectatS.
cerevisiaetelomeres:reversiblerepresssionofPolIItranscription.
Cell1990;63:751-762.
9BaurJA,ZouY,ShayJW,WrightWE.
Telomerepositionef-fectinhumancells.
Science2001;292:2075-2077.
10KoeringCE,PolliceA,ZibellaMP,etal.
Humantelomericpositioneffectisdeterminedbychromosomalcontextandte-lomericchromatinintegrity.
EMBORep2002;3:1055-1061.
11OttavianiA,GilsonE,MagdinierF.
Telomericpositioneffect:fromtheyeastparadigmtohumanpathologiesBiochimie2008;90:93-107.
12BlascoMA.
Theepigeneticregulationofmammaliantelom-eres.
NatRevGenet2007;8:299-309.
13DengZ,NorseenJ,WiedmerA,RiethmanH,LiebermanPM.
TERRARNAbindingtoTRF2facilitatesheterochromatinformationandORCrecruitmentattelomeres.
MolCell2009;35:403-413.
14Ruiz-HerreraA,NergadzeSG,SantagostinoM,GiulottoE.
Telomericrepeatsfarfromtheends:mechanismsoforiginandroleinevolution.
CytogenetGenomeRes2008;122:219-228.
15AzzalinCM,NergadzeSG,GiulottoE.
Humanintrachro-mosomaltelomeric-likerepeats:sequenceorganizationandmechanismsoforigin.
Chromosoma2001;110:75-82.
16AmbrosiniA,PaulS,HuS,RiethmanH.
Humansubtelomer-icdupliconstructureandorganization.
GenomeBiol2007;8:R151.
17NergadzeSG,SantagostinoMA,SalzanoA,MondelloC,GiulottoE.
ContributionoftelomeraseRNAretrotranscrip-tiontoDNAdouble-strandbreakrepairduringmammaliangenomeevolution.
GenomeBiol2007;8:R260.
18IjdoJW,BaldiniA,WardDC,ReedersST,WellsRA.
Originofhumanchromosome2:anancestraltelomere-telomerefu-sion.
ProcNatlAcadSciUSA1991;88:9051-9055.
19BradshawPS,StavropoulosDJ,MeynMS.
Humantelo-mericproteinTRF2associateswithgenomicdouble-strandbreaksasanearlyresponsetoDNAdamage.
NatGenet2005;37:193-197.
20DengZ,LezinaL,ChenCJ,etal.
TelomericproteinsregulateepisomalmaintenanceofEpstein-Barrvirusoriginofplasmidreplication.
MolCell2002;9:493-503.
21ZhangP,PazinMJ,SchwartzCM,etal.
NontelomericTRF2-RESTinteractionmodulatesneuronalgenesilencingandfateoftumorandstemcells.
CurrBiol2008;18:1489-1494.
22TeoH,GhoshS,LueschH,etal.
Telomere-independentRap1isanIKKadaptorandregulatesNF-kappaB-dependentgeneexpression.
NatCellBiol2010;12:758-767.
23SmogorzewskaA,vanSteenselB,BianchiA,etal.
ControlofhumantelomerelengthbyTRF1andTRF2.
MolCellBiol2000;20:1659-1668.
24KrutilinaRI,SmirnovaAN,MudrakOS,etal.
Protectionofinternal(TTAGGG)nrepeatsinChinesehamstercellsbytelo-mericproteinTRF1.
Oncogene2003;22:6690-6698.
25Mignon-RavixC,DepetrisD,DelobelB,CroquetteMF,Mat-teiMG.
AhumaninterstitialtelomereassociatesinvivowithspecificTRF2andTIN2proteins.
EurJHumGenet2002;10:107-112.
26YeJ,LenainC,BauwensS,etal.
TRF2andapollocooperatewithtopoisomerase2alphatoprotecthumantelomeresfromreplicativedamage.
Cell2010;142:230-242.
27MartinezP,ThanasoulaM,CarlosAR,etal.
MammalianRap1controlstelomerefunctionandgeneexpressionthroughbindingtotelomericandextratelomericsites.
NatCellBiol2010;12:768-780.
28JothiR,CuddapahS,BarskiA,CuiK,ZhaoK.
Genome-wideidentificationofinvivoprotein-DNAbindingsitesfromChIP-Seqdata.
NucleicAcidsRes2008;36:5221-5231.
29EdgarR,DomrachevM,LashAE.
GeneExpressionOmni-bus:NCBIgeneexpressionandhybridizationarraydatare-pository.
NucleicAcidsRes2002;30:207-210.
30DesmazeC,AlbertiC,MartinsL,etal.
Theinfluenceofin-terstitialtelomericsequencesonchromosomeinstabilityinhumancells.
CytogenetCellGenet1999;86:288-295.
31MondelloC,PirzioL,AzzalinCM,GiulottoE.
Instabilityofinterstitialtelomericsequencesinthehumangenome.
Ge-nomics2000;68:111-117.
32LeeC,WevrickR,FisherRB,Ferguson-SmithMA,LinCC.
HumancentromericDNAs.
HumGenet1997;100:291-304.
ExtratelomericbindingofTRF1andTRF21038npgCellResearch|Vol21No7|July201133JohnsonDS,MortazaviA,MyersRM,WoldB.
Genome-widemappingofinvivoprotein-DNAinteractions.
Science2007;316:1497-1502.
34YangD,XiongY,KimH,etal.
Humantelomericproteinsoccupyselectiveinterstitialsites.
CellRes2011Mar22.
doi:10.
1038/cr.
2011.
3935SfeirA,KosiyatrakulST,HockemeyerD,etal.
MammaliantelomeresresemblefragilesitesandrequireTRF1forefficientreplication.
Cell2009;138:90-103.
36MartínezP,ThanasoulaM,MuozP,etal.
IncreasedtelomerefragilityandfusionsresultingfromTRF1deficienciesleadtodegenerativepathologiesandincreasedcancerinmice.
GenesDev2009;23:2060-2075.
37MailletL,BoscheronC,GottaM,etal.
Evidenceforsilenc-ingcompartmentswithintheyeastnucleus:arolefortelomereproximityandSir-proteinconcentrationinsilencer-mediatedrepression.
GenesDev1996;10:1796-1811.
38MarcandS,BuckSW,MorettiP,GilsonE,ShoreD.
Silenc-ingofgenesatnontelomericsitesinyeastiscontrolledbyse-questrationofsilencingfactorsattelomeresbyRap1protein.
GenesDev1996;10:1297-1309.
39BaileyTL,ElkanC.
Fittingamixturemodelbyexpectationmaximizationtodiscovermotifsinbiopolymers.
ProcIntConfIntellSystMolBiol1994;2:28-36.
40BlahnikKR,DouL,O'GeenH,etal.
Sole-Search:aninte-gratedanalysisprogramforpeakdetectionandfunctionalannotationusingChIP-seqdata.
NucleicAcidsRes2010;38:e13.
41JurkaJ,KapitonovVV,PavlicekA,etal.
RepbaseUpdate,adatabaseofeukaryoticrepetitiveelements.
CytogenetGenomeRes2005;110:462-467.
42HuangdaW,ShermanBT,LempickiRA.
SystematicandintegrativeanalysisoflargegenelistsusingDAVIDbioinfor-maticsresources.
NatProtoc2009;4:44-57.
(SupplementaryinformationislinkedtotheonlineversionofthepaperontheCellResearchwebsite.
)
妮妮云,美国cera CN2线路,VPS享3折优惠
近期联通CUVIP的线路(AS4837线路)非常火热,妮妮云也推出了这类线路的套餐以及优惠,目前到国内优质线路排行大致如下:电信CN2 GIA>联通AS9929>联通AS4837>电信CN2 GT>普通线路,AS4837线路比起前两的优势就是带宽比较大,相对便宜一些,所以大家才能看到这个线路的带宽都非常高。妮妮云互联目前云服务器开放抽奖活动,每天开通前10台享3折优惠,另外...
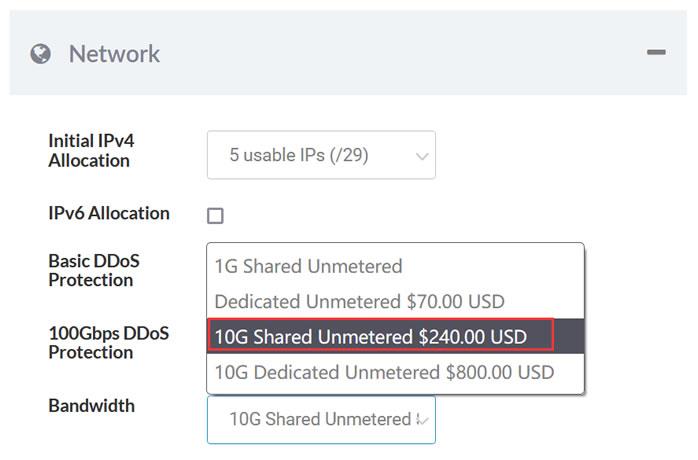
Sharktech10Gbps带宽,不限制流量,自带5个IPv4,100G防御
Sharktech荷兰10G带宽的独立服务器月付319美元起,10Gbps共享带宽,不限制流量,自带5个IPv4,免费60Gbps的 DDoS防御,可加到100G防御。CPU内存HDD价格购买地址E3-1270v216G2T$319/月链接E3-1270v516G2T$329/月链接2*E5-2670v232G2T$389/月链接2*E5-2678v364G2T$409/月链接这里我们需要注意,默...
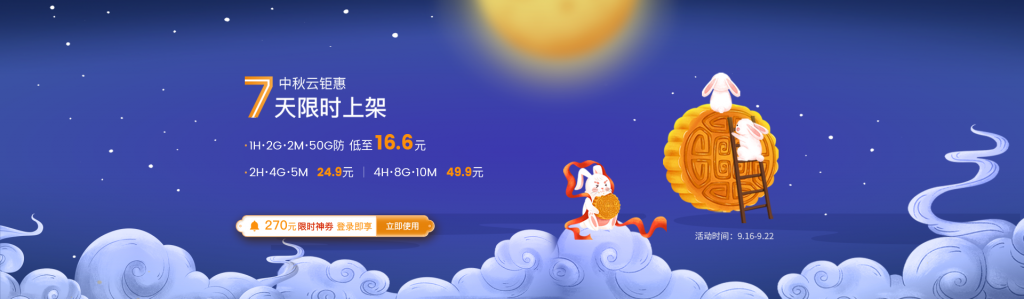
萤光云(16元/月)高防云服务器自带50G防御
螢光云官網萤光云成立于2002年,是一家自有IDC的云厂商,主打高防云服务器产品。在国内有福州、北京、上海、台湾、香港CN2节点,还有华盛顿、河内、曼谷等海外节点。萤光云的高防云服务器自带50G防御,适合高防建站、游戏高防等业务。本次萤光云中秋云活动简单无套路,直接在原有价格上砍了一大刀,最低价格16元/月,而且有没有账户限制,新老客户都可以买,就是直接满满的诚意给大家送优惠了!官网首页:www....
u998为你推荐
-
宕机宕机 这个词是什么意思啊云挂机云挂机每天2+元你提了吗?网络虚拟机虚拟机网络设置网络虚拟机VMware虚拟机三种网络模式的区别有哪些?去鼠标加速度CS去鼠标加速度和鼠标灵敏度的区别?网页打不开的原因为什么我的网页打不开关闭qq相册图标怎样熄灭QQ相册图标怎么把网页的字变大如何使网页的字体变大?av终结者专杀工具AV终结者专杀工具不能删除,怎么办msn与qqMSN与QQ的区别?